Japanese macaque
TAXONOMY
Suborder: Haplorrhini Infraorder: Simiiformes Superfamily: Cercopithecoidea Family: Cercopithecidae Subfamily: Cercopithecinae Genus: Macaca Species: M. fuscata Subspecies: M. f. fuscata, M. f. yakui Other names: Japanese macaque, Japanese monkey, Snow monkey; macaque japonais, macaque à face rouge (French); japansk makak (Swedish); macaca japonesa (Spanish); Nihon zaru (Japanese) (for vernacular names see Fooden & Aimi 2005:77); M. fuscata yakui: Yaku monkey; Yakushimazaru, Yakuzaru (Japanese).MORPHOLOGY

Macaca fuscata
RANGE
CURRENT RANGE MAPS (IUCN REDLIST): Macaca fuscata The Japanese macaque is native to the islands of Japan. Of the four main Japanese islands, Hokkaido, Honshu, Shikoku, and Kyushu, Japanese macaques are found on all but Hokkaido, the northernmost (Fooden & Aimi 2005). Even though its range is restricted to the three southern main islands of Japan, the species nevertheless represents the northernmost wild populations of non-human primates in the world. The absolute northernmost Japanese macaque populations are found at the northern tip of the island of Honshu on the Shimokita peninsula (Izawa & Nishida 1963; Uehara 1975). These northern populations exhibit significant cold adaptation as northern Honshu can be snowbound for up to a third of the year (Izawa & Nishida 1963). Japanese macaques also inhabit several smaller islands near the coasts of Honshu, Shikoku, and Kyushu (Fooden & Aimi 2005). The southernmost population of Japanese macaques is that on Yakushima Island off of the south coast of Japan and has been assigned its own subspecies, M.f.yakui (Uehara 1975; Hanya 2004). In February 1972, a complete group of Japanese macaques numbering 150 individuals was transplanted from Arashiyama, near Kyoto on Honshu to Laredo, Texas where it was established in an arid brushland habitat and grew, having reached 470 individuals by 1989 (Fedigan 1991). The total population of Japanese macaques has been estimated to be 114,431 individuals and likely numbers around 100,000 individuals in its natural habitat (Hashiba 1989; Fooden & Aimi 2005). The Japanese macaque is rarely found in lowland areas owing to the high levels of human habitation in those areas (Amagasa & Ito 1978 cited in Fooden & Aimi 2005). The Japanese macaque has been studied in the wild longer than most primate species, having been observed in numerous habitats and locations throughout Japan for over 50 years (Yamagiwa & Hill 1998). Since the 1950’s, study of Japanese macaques has been undertaken at Arashiyama, near Kyoto (Huffman 1991a). This long-term study site has not only served to provide information as to the long-term changes within a Japanese macaque population, but also to serve as the source of the introduced Arashiyama West troop in Texas which has provided not only a study site for the Japanese macaque in north America, but a place to study adaptations of the species to a new habitat (Fedigan 1991). Within their range, the distribution of the Japanese macaque is expanding, at least partially as a result of the species losing their fear of humans, coupled with demographic and economic shifts in the Japanese human population (Watanabe & Muroyama 2005). This expansion may be misleading as to the status of the species however, because within the range, the total population is significantly limited by the distribution of the natural broadleaf forest that is available. In addition, the expansion of the range distribution was found to be correlated with the reduction of forests (Hashiba 1989).HABITAT
Due to variations in the latitude and altitude of the Japanese islands, the habitat of the Japanese macaque varies greatly between the extremes of its distribution. Near the southern end of the population distribution, habitats include sub-tropical forest and at the northernmost reaches, sub-arctic forest is found in mountainous regions. Between these two extremes, both warm and cool temperate forests are found (Uehara 1975). These types of forest include both the deciduous forests of central and northern Japan and the broadleaf evergreen forests of the southwest of the islands. As is expected in a variable range, there is a large spectrum of vegetation within the distribution of the Japanese macaque (Suzuki 1965). The highest elevation at which the Japanese macaque has been reported is 3180 m (10,433 ft) (Izumiyama pers. comm. cited in Fooden & Aimi 2005). Of the habitats of the Japanese macaque, the two most important are the warm temperate evergreen broadleaf forest and the cool temperate deciduous broadleaf forest (Fooden & Aimi 2005). In the northern deciduous forests, leaves are absent from the trees for up to 5 months of the year (Suzuki 1965). Near the northern end of the range in the cool temperate deciduous broadleaf forest on the island of Kinkazan, annual rainfall averages 1500mm (59.06 in) with an average temperature of 11° C (51.8° F). At the extreme southern end of the macaque range on the island of Yakushima in warm temperate evergreen broadleaf forest, annual rainfall averages 3000mm (118.11 in) with an average temperature of 20° C (68° F). During the winter in high altitude or latitude areas of the Japanese macaque range, snow is often quite deep, having been recorded on the Shimokita peninsula and in the Shiga Heights in central Honshu to be between 2-3 meters deep during the winter (Izawa & Nishida 1963; Hori et al. 1977).ECOLOGY

Macaca fuscata

Macaca fuscata
Content last modified: April 26, 2007
Written by Kurt Gron. Reviewed by Sarah Turner.
Cite this page as: Gron KJ. 2007 April 26. Primate Factsheets: Japanese macaque (Macaca fuscata) Taxonomy, Morphology, & Ecology . <http://pin.primate.wisc.edu/factsheets/entry/japanese_macaque/taxon>. Accessed 2020 July 21.
SOCIAL ORGANIZATION AND BEHAVIOR
Japanese macaque groups are matrilineal groups (Fooden & Aimi 2005). Female Japanese macaques remain with their natal groups for life while males emigrate before becoming sexually mature (Fukuda 2004). Groups are typically multi-male and multi-female populated with several males which have immigrated from other groups and females, still in their natal group (Fukuda 2004). Several, and often many, matrilines can be present in a single Japanese macaque troop. In a troop it is possible to arrange kin groups according to rank on a linear continuum (Koyama 1967). Thus, all of the members of a specific kin group are higher ranked than all of the members of a lower-ranked kin group. Group composition averages around 18% adult males, 32% adult females, 35% juveniles, and 15% infants (Fooden & Aimi 2005). Males typically emigrate from their natal group between five or six years of age and sometimes form temporary all male groups (Fukuda 2004). Males which have emigrated often join and leave groups several times in their lives and may stay in a new troop for years (Fukuda 1982 cited in Fukuda 2004). These new groups can be considerably far away from the male’s natal group, and in exceptional cases, involving travel surpassing 100km (62.14 mi) to reach (Yoshimi & Takasaki 2003). In fact, many males spend a significant amount of their lives outside of membership in any group (Sugiyama 1976).
Macaca fuscata
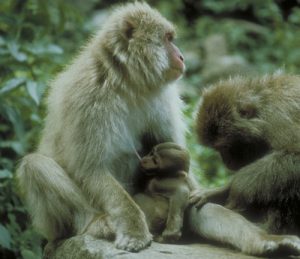 There are three different ways in which troops of Japanese macaques experience social change. These are troop fission, or division; takeover of control by a new alpha-male; and extinction, in which the troop ceases to exist (Maruhashi 1992). Most social changes within troops of Japanese macaques occur as a result of interplay between the mating strategies of both male and female members of the troop vying for reproductive advantage (Maruhashi 1992). Fission in groups helps to control group size, maintain male hierarchies, and to possibly limit inbreeding (Furuya 1969).
Grooming plays an important role in female social organization. In Japanese macaques, as in other primates, grooming serves to reinforce social bonds and friendly social relationships between individuals, in addition to serving hygienic purposes (Majolo et al. 2005). There is a strong correlation in grooming between pairs who are matrilineally related as opposed to unrelated individuals (Koyama 1991). However, grooming among individuals who are unrelated does occur and serves to reinforce group cohesion as a whole as it strengthens bonds between different kin groups within a troop (Nakamichi & Shizawa 2003). Females tend to groom only a small cohort of other females, even if group size increases (Nakamichi & Shizawa 2003). Allogrooming of other individuals by the Japanese macaque is independent of climate and season differences, which supports the view that its function is primarily social (Ventura et al. 2005). When males are groomed by females, it is likely for skin-care purposes but helps the females attract and retain high-ranking males in the troop for reproductive purposes (Tsukahara 1990). Grooming techniques are passed from mother to offspring, probably through social means and not genetically (Tanaka 1995).

Macaca fuscata
REPRODUCTION
A key feature of the reproduction of the Japanese macaque is the consortship . This association between a male and a female Japanese macaque is characterized by a pair mating, feeding, resting, and traveling together, and lasts an average of 1.6 days during mating season (Huffman 1992). Over the course of a mating season, Japanese macaque females were observed to enter consortships with over 4 different males on average (Gouzoules & Goy 1983). Typically there is a correlation between male rank and consort duration, with higher-ranking males remaining in consortships longer than lower-ranking males (Huffman 1992). Higher-ranking males will interfere in the consortships of lower-ranking males in an attempt to disrupt them (Perloe 1992). Females attempt to mate with males of all ranks, but are more likely to actually mate with higher ranking males due to their ability to mate-guard and aggressively prevent mating with lower-ranking males (Soltis 1999). Ultimately, it is the female who makes the decision as to whether or not mating will occur (Huffman 1991b). There is some ambiguity as to whether or not an ultimate correlation exists between male dominance rank and ultimate reproductive success, but male dominance rank does not ensure mating opportunities with receptive females (Fooden & Aimi 2005). In addition, females will typically mate with more than one male during an estrus season (Matsubara & Sprague 2004). Finally, a significant number of copulations by females are with non-troop males who enter the troop during mating season and then depart after the season (Sprague 1991).
Macaca fuscata
PARENTAL CARE
To give birth, a Japanese macaque mother will move to the periphery of the troop and to a private spot (Fedigan & Zohar 1997). However, if the troop moves during birth, the mother will move to remain with the group and will not allow herself to be separated from it (Nakamichi et al. 1992; Thomsen 1997). Birth in the wild typically takes place on the ground (Fooden & Aimi 2005). Infant mortality before one year averages 28.4% in wild groups of Japanese macaques (Fooden & Aimi 2005). Weight at birth for Japanese macaque infants averages 546.8 g (1.21 lbs) for females and 538.7 g (1.19 lbs) for males (Fooden & Aimi 2005). At birth, the fur of the infant Japanese macaque is very dark brown and lightens progressively over the next six months while still remaining somewhat darker than the coat of the adult during that time (Hiraiwa 1981). Solid food consumption by the infant is first seen at 5 or 6 weeks of age followed by foraging independent of the mother at 7 weeks of age (Hiraiwa 1981). From birth until 4 weeks, an infant is carried ventrally by the mother. After 4 weeks of age, dorsal carrying is observed in addition to ventral carrying. Carrying by the mother can persist up to and past one year of age (Hiraiwa 1981).
Macaca fuscata
COMMUNICATION
The Japanese macaque utters a number of vocalizations which can be roughly divided into six groups: peaceful or soothing, defensive, aggressive, warning, female estrus, and infant vocalizations (Itani 1963). Over half of the vocalizations uttered by the Japanese macaque are peaceful or calm (Itani 1963). Often, during feeding or moving, Japanese macaques will utter a “coo” sound which likely functions in group cohesion by allowing females to reinforce their social ties (Mitani 1986). This “coo” sound is not typically heard in agonistic interactions, and when uttered, other Japanese macaques typically respond in kind (Sugiura 2001).
Macaca fuscata
Content last modified: April 26, 2007
Written by Kurt Gron. Reviewed by Sarah Turner.
Cite this page as: Gron KJ. 2007 April 26. Primate Factsheets: Japanese macaque (Macaca fuscata) Behavior . <http://pin.primate.wisc.edu/factsheets/entry/japanese_macaque/behav>. Accessed 2020 July 21.
INTERNATIONAL STATUS
For individual primate species conservation status, please search the IUCN Red List. Also search the current scientific literature for primate conservation status (overall as well as for individual species), and visit CITES (Convention on International Trade in Endangered Species of Wild Fauna and Flora).
Macaca fuscata
CONSERVATION THREATS
Threat: Human Induced Habitat Loss and Degradation
The Japanese macaque has arrived at somewhat of a crossroads in relation to its conservation and the threats to its survival. Since the Second World War, traditional threats to the species such as slash-and-burn agriculture, use of forest woods for construction and fuel, and hunting decreased significantly, mainly due to social and economic changes in Japan (Sprague 2002). In this regard, the outlook for conservation of the Japanese macaque looks significantly brighter. On the other hand, with such a shift from traditional threats, new conflicts with the species have emerged. The two most serious of these new threats are the replacement of natural forests with lumber plantations and the rise in crop-raiding by the Japanese macaque (Sprague 2002). The lumber plantations cannot be used as habitat by the monkeys and the rise in crop-raiding has resulted in the species being considered a nuisance. Behind wild boar and deer, the Japanese macaque is the third worst crop-raider in Japan (Sprague 2002). As a result, they have less appropriate habitat in which to live coupled with yearly culling of the species as a pest in excess of 10,000 individuals per annum (Watanabe & Muroyama 2005). Apparently, the range of the species is expanding but whether or not the total number of Japanese macaques is expanding or contracting is unclear. The range expansion is attributed to behavioral changes within the Japanese macaque population in which they have lost their fear of humans and do not actively avoid people (Watanabe & Muroyama 2005). This lack of fear has resulted in a Japanese macaque presence in not only rural and agricultural areas, but an increasing presence in urban areas. In one extreme case, a female was living in central Tokyo for several months (Fukuda 2004). In 1993, part of Yakushima island, the habitat of M. f. yakui, was designated a Natural World Heritage Site by UNESCO which has proven to have had mixed results for conservation at that locale (Hill & Maruhashi 1996/1997). The designation, while raising awareness of a need for conservation, has brought additional tourists to the threatened habitat and has not as of yet proven adequate for protection of the Japanese macaques of Yakushima island (Hill & Maruhashi 1996/1997).LINKS TO MORE ABOUT CONSERVATION
CONSERVATION INFORMATION
- No current links for Macaca fuscata
- Links for all species
CONSERVATION NEWS
- Look, but don’t stare! Hanging out with Kyoto’s macaques (CNN; May 9, 2013)
- Links for all species
ORGANIZATIONS INVOLVED IN Macaca fuscata CONSERVATION
Content last modified: April 26, 2007
Written by Kurt Gron. Reviewed by Sarah Turner.
Cite this page as: Gron KJ. 2007 April 26. Primate Factsheets: Japanese macaque (Macaca fuscata) Conservation . <http://pin.primate.wisc.edu/factsheets/entry/japanese_macaque/cons>. Accessed 2020 July 22.
REFERENCES
Aetsuma N, Nakagawa N. 1998. Effects of habitat differences on feeding behaviors of Japanese monkeys: comparison between Yakushima and Kinkazan. Primates 39(3):275-89. Bardi M, Shimizu K, Fujita S, Borgognini-Tarli S, Huffman MA. 2001. Social behavior and hormonal correlates during the perinatal period in Japanese macaques. Horm Behav 39(3):239-46. Blount B. 1985. “Girney” vocalizations among Japanese macaque females: context and function. Primates 26(4):424-35. Chatani K. 2003. Positional behavior of free-ranging Japanese macaques (Macaca fuscata). Primates 44(1):13-23. Eaton G. 1972. Snowball construction by a feral troop of Japanese macaques (Macaca fuscata) living under seminatural conditions. Primates 13(4):411-4.
Macaca fuscata

Macaca fuscata
Content last modified: April 26, 2007
VIDEO & WEBCAMS
- Snow Monkeys (3:02, narrated; National Geographic Kids; Flash)
- Wet ‘n’ Wild (1:12, narrated; National Geographic Kids; Flash)
IMAGES
 |
Macaca fuscata Photo: Alisha Eisert |
 |
Macaca fuscata Photo: Alisha Eisert |
 |
Macaca fuscata Photo: Alisha Eisert |
 |
Macaca fuscata Photo: Alisha Eisert |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Frans de Waal |
 |
Macaca fuscata Photo: Marilyn Cole |
Primate Info Net (PIN) is maintained by the Wisconsin National Primate Research Center (WNPRC) at the University of Wisconsin-Madison, with countless grants and contributions from others over time. PIN is an ever-growing community effort: if you’d like to contribute, or have questions, please don’t hesitate to contact us.